Hadee Thompson‑Morrison 1,3*, Fransisca Ariantiningsih 2, Sugesti Muhammad Arief 2, Sally Gaw 1 & Brett Robinson 1
The production of oil palm (Elaeis guineensis) in Southeast Asia is vital to the economies of Indonesia and Malaysia. Both fertilisers and pesticides used in palm production can contain elevated concentrations of Trace Elements (TEs) which may accumulate in soils and leaf tissues of plants. We hypothesised that leaves from oil palms may be deficient in essential elements, while containing elevated concentrations of non‑essential TEs commonly found in agrichemicals. Samples of plant materials (leaves and fruitlets) were collected from active and former plantations in Sumatra, Indonesia, and analysed for essential and non‑essential elements. Indonesian palm oil samples were sourced in New Zealand and their elemental concentrations determined. Leaf materials from both active and abandoned production sites were deficient in N, K, S and Mo, while leaf materials from abandoned sites were deficient in P. These deficiencies may have been a contributing factor to the abandonment of production at these sites. Concentrations of non‑essential elements were below or comparable to average plant concentrations and no evidence of contamination was found in plant tissues. Palm oil contained low concentrations of TEs, which did not pose any toxicity risks. However, Na and Al were present in concentrations of 1198 and 159 mg kg−1 respectively, which were higher than have been previously reported. Tropical oil palm production could benefit from the determination of bioaccumulation factors for fertiliser contaminants in E. guineensis, to limit the transfer of contaminants to plants and products if increased fertiliser applications were used to correct nutrient deficiencies.
东南亚的油棕(Elaeis guineensis)生产对印度尼西亚和马来西亚的经济至关重要。油棕生产中使用的化肥和农药均可能含有较高浓度的微量元素(TEs),这些元素可能在土壤和植物叶片组织中累积。我们假设油棕叶片可能缺乏必需元素,同时含有农用化学品中常见的高浓度非必需微量元素。本研究在印度尼西亚苏门答腊的在产及废弃种植园采集植物材料(叶片和小果)样品,分析其中的必需元素和非必需元素;并在新西兰购得印度尼西亚棕榈油样品,测定其元素浓度。在产和废弃生产地的叶片材料均缺乏N、K、S和Mo,而废弃地的叶片材料还缺乏P。这些缺乏可能是上述生产地被废弃的原因之一。非必需元素浓度低于或相当于植物平均浓度,植物组织中未发现污染迹象。棕榈油中微量元素浓度较低,不构成任何毒性风险。然而,Na和Al的浓度分别为1198和159 mg kg−1 ,高于以往报道的水平。若为纠正养分缺乏而增加施肥量,热带油棕生产可通过测定肥料污染物在E. guineensis中的生物累积系数而受益,从而限制污染物向植物及其产品的迁移。
The African oil palm (Elaeis guineensis Jacq.) is an economically important crop, producing the world’s most consumed vegetable oil1. Palm oil represents 10% of Indonesia’s exports and 5% of Malaysia’s, with these two countries being the world’s major cultivators of E. guineensis2. A 2016 assessment determined that 45% of harvested E. guineensis plantation land in Southeast Asia had been converted from tropical forests since 19893. Tropical forest soil is typically nutrient-poor and requires inputs of both capital and maintenance nutrients through fertilisers to support production4,5. The essential elements of most importance for E. guineensis are N, P, K, Mg and B6. Inadequate supply of these elements through fertilisers can lead to yield reductions in E. guineensis production, particularly on acidic and weathered tropical soils such as those from Indonesia and Malaysia6,7. Plant deficiencies can be assessed through the leaf concentrations of essential elements.
非洲油棕(Elaeis guineensis Jacq.)是一种具有重要经济价值的作物,其所产植物油是全球消费量最大的植物油1。棕榈油占印度尼西亚出口额的10%和马来西亚出口额的5%,这两个国家是全球E. guineensis的主要种植国2。2016年的一项评估表明,东南亚已收获的E. guineensis种植园土地中,有45%是自1989年以来由热带森林转化而来的3。热带森林土壤通常养分贫瘠,需通过施肥投入基础养分和维持养分以支撑生产4,5。对E. guineensis最为重要的必需元素为N、P、K、Mg和B6。施肥对这些元素的供应不足会导致E. guineensis减产,在印度尼西亚和马来西亚等地的酸性、强风化热带土壤上尤为明显6,7。植物养分缺乏可通过叶片中必需元素的浓度进行评估。
Fertiliser-borne trace elements (TEs) can accumulate in soil to concentrations that exceed guideline values8. Pesticides and other agrichemicals used to support production are also potential sources of TEs6,9,10. If soil-accumulated TEs are taken up by plants, this has potential for products to exceed food safety standards8,11. The transfer of TEs into plant products is a function of plant TE uptake, surface deposition and post-harvest contamination. The root absorption of TE ions in soil solution occurs via the symplastic and apoplastic pathways, followed by xylem transport to leaves and potential phloem transport to fruit tissues12. Spray residues containing TEs can sorb to plant leaves after direct pesticide applications, while deposition of soil containing TEs onto plant parts used for manufacturing can lead to plant products containing TEs13. Trace elements can also enter products due to contamination from machinery and equipment during manufacturing, processing and storage post-harvest14,15. The uptake of ions from soil solution is governed by its bioavailability: high total concentrations of TEs in soil do not always correspond with high uptake16. Bioavailability is a function of the solubility and speciation of the TE in soil, the presence of competing ions as well as the receptor organism12. Leaf concentrations—particularly pinnae concentrations in E. guineensis—of essential elements are better indicators of plant nutrition than the total soil concentration17. The presence of TEs in vegetable oils as a result of plant uptake and transport is typically limited due to their partitioning away from the lipid phase in plants18. This is supported by no identification of concentrations of TEs in processed palm oils at which breached food safety standards19. Although some TEs may be present in crude palm oil, these are removed during refining processes20–22.
肥料带入的微量元素(TEs)可在土壤中累积至超过指导限值的浓度8。用于支撑生产的农药及其他农用化学品也是微量元素的潜在来源6,9,10。若土壤中累积的微量元素被植物吸收,则产品可能超出食品安全标准8,11。微量元素向植物产品的迁移取决于植物对微量元素的吸收、表面沉降以及采后污染。根系对土壤溶液中微量元素离子的吸收经由共质体和质外体途径进行,随后通过木质部运输至叶片,并可能经韧皮部运输至果实组织12。直接施用农药后,含微量元素的喷雾残留物可吸附于植物叶片;而含微量元素的土壤沉降在用于加工的植物部位上,也可导致植物产品中含有微量元素13。在采后加工、处理和储存过程中,机械和设备的污染亦可使微量元素进入产品14,15。植物对土壤溶液中离子的吸收受其生物有效性控制:土壤中微量元素总浓度高并不总是对应于高吸收量16。生物有效性取决于微量元素在土壤中的溶解度和形态、竞争离子的存在以及受体生物12。相比土壤总浓度,叶片中必需元素的浓度(尤其是E. guineensis的羽片浓度)能更好地指示植物营养状况17。由于微量元素在植物体内倾向于分配到脂相之外,经植物吸收和运输而进入植物油的微量元素通常有限18。这一点得到以下事实的支持:尚未发现加工棕榈油中微量元素浓度超出食品安全标准的情况19。尽管粗棕榈油中可能含有某些微量元素,但它们在精炼过程中被去除20–22。
1School of Physical and Chemical Sciences, University of Canterbury, Christchurch, New Zealand. 2Orangutan Information Centre, Medan, Sumatra, Indonesia. 3Present address: Manaaki Whenua Landcare Research, Lincoln, New Zealand. *email: Thompson-MorrisonH@landcareresearch.co.nz
Concurrent research on E. guineensis plantation soils from Indonesia23 determined that the soils analysed were deficient in essential nutrients N, P, K, Mg and Mo, and elevated above background levels in TEs Cu, Zn, As and Pb. Furthermore, the soils analysed were acidic and TEs were more mobile compared to other arable systems. In the current work, we analysed E. guineensis plant materials—leaves, rachides, endosperms and mesocarps—from the same plantations as well as the E. guineensis product palm oil for with a specific focus on plant-essential nutrient and TE composition.
同期对印度尼西亚E. guineensis种植园土壤的研究23表明,所分析土壤缺乏必需养分N、P、K、Mg和Mo,而微量元素Cu、Zn、As和Pb高于背景水平。此外,所分析土壤呈酸性,与其他耕作系统相比微量元素的迁移性更强。在本研究中,我们分析了采自相同种植园的E. guineensis植物材料(叶片、叶轴、胚乳和中果皮)以及E. guineensis产品棕榈油,重点关注植物必需养分和微量元素的组成。
We hypothesise that E. guineensis leaf concentrations of N, P, K, Mg and Mo will be deficient and below concentrations of 2.3%, 1400 mg kg-1, 7500 mg kg-1, 2000 mg kg-1 and 0.3 mg kg-1, respectively. Furthermore, we hypothesise that concentrations of Cu, Zn, As and Pb may be elevated in plant tissues. We hypothesise that palm oil will contain inconsequential levels of all elements below tolerable upper limits for food safety. This research aims to determine whether plants are deficient in essential nutrients and elevated in TEs, and thus the benefits and risks of using E. guineensis products with specific respect to chemical elements.
我们假设E. guineensis叶片中N、P、K、Mg和Mo的浓度处于缺乏状态,分别低于2.3%、1400 mg kg-1、7500 mg kg-1、2000 mg kg-1和0.3 mg kg-1。此外,我们假设植物组织中Cu、Zn、As和Pb的浓度可能升高。我们还假设棕榈油中所有元素的含量均微不足道,低于食品安全的可耐受最高摄入量。本研究旨在确定植物是否缺乏必需养分且微量元素含量升高,进而明确就化学元素而言使用E. guineensis产品的益处与风险。
1Methods方法
Site descriptions and sample collection样地描述与样品采集
Plant material samples were collected from three E. guineensis plantations in Sumatra, Indonesia in May 2019. All plantations shared a common soil type of Acrisol (taxonomically related to Oxisols according to the USDA soil classification24). The sampling locality (approximately 3.5952° N, 98.6722° E) is reported in Thompson-Morrison et al.23. Materials collected included leaves, rachides and whole kernels, which were divided into mesocarp and endosperm prior to analysis. Plant material was cleaned with water and oven dried at 60 °C until a constant weight was obtained. All samples were ground prior to analysis.
植物材料样品于2019年5月采自印度尼西亚苏门答腊的三个E. guineensis种植园。所有种植园的土壤类型均为强淋溶土(Acrisol,按美国农业部土壤分类与氧化土在分类学上相关24)。采样地点(约3.5952° N, 98.6722° E)见Thompson-Morrison et al.23的报道。采集的材料包括叶片、叶轴和完整果核,果核在分析前分为中果皮和胚乳。植物材料用水清洗后于60 °C烘干至恒重。所有样品在分析前均经研磨。
The study was conducted in accordance with the relevant institutional, national, and international guidelines. Permissions were obtained from landowners for the collection of plant material and plants were identified by the landowners or farmers present during sampling. Samples were sent to the University of Canterbury in New Zealand under approved permits from both New Zealand’s Ministry for Primary Industries (permits #2019072466 for kernel material and #2018068845 for leaf material) and Indonesia’s Agency for Agricultural Quarantine (phytosanitary certificate #2019.2.0702.0.K10.E.000785 for kernel material and #2019.2.0702.0.K10.E.000728 for leaf material). Kernels were crushed and ground prior to export to ensure non-viability. Once in New Zealand, samples were stored and analysed in Physical Containment Level 2 approved facilities with kernels stored at ~ 4 °C.
本研究按照相关机构、国家和国际准则开展。采集植物材料前已获得土地所有者许可,植物由采样时在场的土地所有者或农户鉴定。样品经新西兰初级产业部(果核材料许可证号#2019072466,叶片材料许可证号#2018068845)和印度尼西亚农业检疫局(果核材料植物检疫证书号#2019.2.0702.0.K10.E.000785,叶片材料植物检疫证书号#2019.2.0702.0.K10.E.000728)批准许可,寄送至新西兰坎特伯雷大学。果核在出口前经压碎和研磨以确保其丧失活力。样品抵达新西兰后,在经批准的二级物理防护(Physical Containment Level 2)设施中储存和分析,果核储存于约4 °C。
Sites A and B were adjacent but separate sites that both bordered Gunung Leuser National Park and were abandoned after ca. 30 years of production. These sites were adjacent to each other and were separated northeast (Site A)/southwest (Site B). At the time of sampling, the sites were overgrown and had had no amendments applied for at least 3 years and had not been harvested throughout this time period. Previous to this, they were under corporate management and underwent regular harvesting. Sites A and B had slopes of approximately 12° in places and samples were taken based on practicality and accessibility from areas in which E. guineensis trees remained.
样地A和B相邻但彼此独立,均毗邻Gunung Leuser国家公园,在经过约30年的生产后被废弃。两样地相互毗邻,以东北(样地A)/西南(样地B)划分。采样时,样地杂草丛生,已至少3年未施用任何改良剂,期间亦未进行收获。在此之前,两样地由企业管理并定期收获。样地A和B局部坡度约为12°,样品根据可行性和可达性从仍有E. guineensis植株的区域采集。
Site C was also near to Gunung Leuser National Park, however, was an active smallholder E. guineensis plantation. This site had been under production for ca. 20 years. Weeds were regularly cleared from the understory of this plantation using spray chemicals and fruit were regularly harvested. The slope of this site was < 4°.
样地C同样靠近Gunung Leuser国家公园,但为在产的小农户E. guineensis种植园。该样地已生产约20年。种植园林下杂草定期以喷施化学药剂清除,果实定期收获。该样地坡度 < 4°。
Samples of refined palm oil were sourced from an Indonesian food manufacturer whose food products are marketed in New Zealand.
精炼棕榈油样品购自一家印度尼西亚食品生产商,其食品在新西兰销售。
Analytical methods分析方法
Pseudo‑total element concentrations准全量元素浓度
We analysed pseudo-total element concentrations (hereafter referred to as elemental concentrations) of all samples using microwave digestion, following EPA Method 3051A25. A Ultrawave Single Reaction Chamber Microwave Digestion Unit was used. In each analysis, 0.20 g (± 0.01 g) was weighed into a digestion tube and 5 mL 70% HNO3 was added. Samples were pre-digested overnight and then digested in the Ultrawave at 230°C for 25 min26. Two reagent blanks and two standard reference materials27,28 were included with every 11 samples for quality assurance. Digestates were analysed by inductively coupled plasma-mass spectrometry along with standard reference materials29. Recoveries of SRMs ranged from 79–134% of certified values. A full list of SRM recoveries is available in Supplementary Materials Table S1. All concentrations reported are on a dry weight basis. The limit of quantification for analyses was 0.01 mg kg-1.
我们按照EPA Method 3051A25,采用微波消解法测定所有样品的准全量元素浓度(以下简称元素浓度)。所用仪器为Ultrawave单反应腔微波消解系统。每次分析称取0.20 g(± 0.01 g)样品于消解管中,加入5 mL 70% HNO3。样品先预消解过夜,然后在Ultrawave中于230°C消解25 min26。为保证质量,每11个样品中加入两个试剂空白和两个标准参考物质27,28。消解液与标准参考物质一同采用电感耦合等离子体质谱法进行分析29。标准参考物质(SRMs)的回收率为认证值的79–134%。SRM回收率完整列表见补充材料表S1。所有报道浓度均以干重计。分析的定量限为0.01 mg kg-1。
Total carbon and nitrogen全碳和全氮
Total C and N concentrations of all samples were analysed by C and N analyser: CN828 Elemental Analysis by Combustion. Blanks and SRMs30 were included with samples for quality assurance.
所有样品的全C和全N浓度采用C/N分析仪测定:CN828燃烧法元素分析。为保证质量,样品中同时加入空白和标准参考物质30。
Bioaccumulation coefficients生物累积系数
Bioaccumulation coefficients (BACs) give an indication of a plant’s ability to accumulate heavy metals from soils31. They can be calculated as the plant / soil TE concentration quotient for each plant tissue using the equation32
生物累积系数(BACs)可指示植物从土壤中累积重金属的能力31。其可按下式计算为各植物组织中微量元素浓度与土壤中微量元素浓度之商32
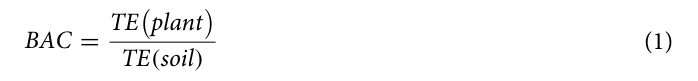
Bioaccumulation coefficients were calculated for pinnae, endosperm and mesocarp tissue from each site. These were calculated for Cu, Zn, As, Sr, Cd and Pb using soil concentrations from these sites detailed in Thompson-Morrison et al.23. These TEs were chosen as they are common contaminants of agrichemicals used to support production33.
计算了各样地羽片、胚乳和中果皮组织的生物累积系数。利用Thompson-Morrison et al.23报道的这些样地的土壤浓度,计算了Cu、Zn、As、Sr、Cd和Pb的生物累积系数。选择这些微量元素是因为它们是用于支撑生产的农用化学品中的常见污染物33。
Statistical Analysis统计分析
R (version 4.1.0) was used for all statistical analysis34. One-way parametric Analysis of Variance (ANOVA) was run to compare means of each sample type between site using the package multcomp35. Data was (natural) logtransformed where assumptions of normality were not met and non-parametric permutational ANOVA was used when assumptions of homoscedacity were not met. In most cases there were no differences between the results of the parametric and non-parametric ANOVA and the parametric test was considered robust. When significant differences were identified, Tukey’s Honest Significant Difference test was run to determine which sites these existed between.
所有统计分析均采用R(4.1.0版)进行34。利用multcomp程序包35进行单因素参数方差分析(ANOVA),比较各样品类型在不同样地间的均值。当不满足正态性假设时,对数据进行(自然)对数转换;当不满足方差齐性假设时,采用非参数置换ANOVA。在大多数情况下,参数与非参数ANOVA的结果无差异,故认为参数检验是稳健的。当发现显著差异时,采用Tukey真实显著差异检验确定差异存在于哪些样地之间。
2Results and discussion结果与讨论
Elements in E. guineensis leaves (pinnae and rachides)E. guineensis叶片(羽片和叶轴)中的元素
Essential elements必需元素
Deficiencies of N, K, S and Mo were present in pinnae samples from all sites, whereas P deficiency was present in pinnae samples from abandoned Sites, A and B (Table 1). The leaf tissue samples tended to contain higher concentrations of both essential and non-essential elements compared to fruit (kernel and mesocarp) tissue. This is consistent with plant physiology, given leaves are a water-sink and elements taken up via the roots are transported here via xylem flow12.
所有样地的羽片样品均存在N、K、S和Mo缺乏,而P缺乏出现在废弃样地A和B的羽片样品中(表1)。与果实(果核和中果皮)组织相比,叶片组织样品中必需元素和非必需元素的浓度往往更高。这与植物生理学相符,因为叶片是水分汇,经根系吸收的元素通过木质部流运输至此12。
Mean concentrations of N, S and Mo in pinnae samples were in the deficient range for oil palm production at all sites. In contrast, P was deficient in 100% of samples at both of the abandoned sites (A and B) and mean K was deficient at Sites B and C (Table 1). Nitrogen deficiencies were present in all pinnae samples from the three sites. The mean N concentrations at Site C (1.9%) were comparable to those of palms grown on Malaysian Oxisols of 1.8%14. Across all sites, the N concentrations (1.3–1.9%) were lower than those of oil palms grown in
所有样地羽片样品中N、S和Mo的平均浓度均处于油棕生产的缺乏范围。相比之下,两个废弃样地(A和B)100%的样品缺乏P,而样地B和C的K平均浓度处于缺乏状态(表1)。三个样地的所有羽片样品均存在N缺乏。样地C的平均N浓度(1.9%)与马来西亚氧化土上种植的油棕(1.8%)相当14。在所有样地中,N浓度(1.3–1.9%)均低于种植于
| Site样点 | A (n = 10) * | B (n = 7) | C (pinnae n = 2, rachides n = 1)C(羽片 n = 2, 叶轴 n = 1) | Deficient+缺乏+ | Adequate+适宜+ | Excessive/ toxic+过量/ 毒害+ | ||
|---|---|---|---|---|---|---|---|---|
| C (%) | 48(0.35)a | 47(0.20)a | 48(0.15)a | – | – | – | ||
| N (%) | 1.4(0.090)a | 1.3(0.077)a | 1.9(0.010)b | < 2.3 | 2.4–2.8 | > 3.0 | ||
| Ml | P | 1102(49)a | 1054(27)a | 1689(144)b | < 1400 | 1500–1800 | > 2500 | |
| acro-eements | K | 9266(982)a | 7109(857)a | 5350(249)a | < 7500 | 9000–12,000 | > 16,000 | |
| S | 1729(119)a | 1799(148)a | 1804(24)a | < 2000 | 2500–3500 | > 6000 | ||
| Mg | 3139(376)a | 2883(354)a | 2476(316)a | < 2000 | 2500–4000 | > 7000 | ||
| Pinnae | B | 21(3.1)a | 24(1.8)a | 12(5.5)a | < 8.0 | 15–25 | > 40 | |
| Mn | 272(44)a | 910(197)b | 705(150)ab | < 35 | 50† | 400–1000‡ | ||
| Fe | 83(5.1)a | 80(5.3)a | 68(7.1)a | – | 100† | – | ||
| Micro-elements | Cu | 5.8(0.26)a | 5.9(0.73)a | 7.6(2.2)a | < 3.0 | 5.0–8.0 | > 15 | |
| Zn | 25(1.4)a | 24(1.6)a | 23(0.68)a | < 10 | 12–18 | > 80 | ||
| Mo | 0.13(0.025)ab | 0.060(0.010)a | 0.24(0.040)b | 0.10–0.30‡ | 0.50–0.80 | 10–50‡ | ||
| C (%) | 47(0.14)a | 47(0.19)a | 48a | – | – | – | ||
| N (%) | 0.20(0.024)a | 0.21(0.037)a | 0.61b | – | – | – | ||
| Ml | P | 462(52)a | 687(184)a | 1316a | – | – | – | |
| acro-eements | K | 8969(1760)a | 6204(876)a | 8614a | < 13,000 | 13,100–16,000 | > 16,000 | |
| S | 837(96)a | 998(126)a | 947a | – | – | – | ||
| Mg | 742(145)a | 898(43)a | 1117a | – | – | – | ||
| Rachides | B | 28(4.2)a | 25(5.0)a | 22a | – | – | – | |
| Mn | 35(7.0)a | 132(26)b | 78ab | – | – | – | ||
| Fe | 63(17)a | 61(12)a | 19a | – | – | – | ||
| Micro-elements | Cu | 2.4(0.17)a | 2.3(0.22)a | 2.3a | – | – | – | |
| Zn | 10(1.1)a | 13(2.1)a | 7.8a | – | – | – | ||
| Mo | 0.20(0.048)a | 0.16(0.031)a | 0.020a | – | – | – |
Nigeria (2.1%) and Indonesia (2.3–2.7%)7,14. For the Indonesian palms, 2.3% N was considered deficient. Nitrogen deficiencies have also been reported in oil palms from Cameroon36 and primarily affect leaf production, size, colour and net assimilation rate17. With insufficient N, oil palms will suffer depressed growth which becomes increasingly exacerbated with age17.
尼日利亚(2.1%)和印度尼西亚(2.3–2.7%)的油棕7,14。对于印度尼西亚的油棕,2.3%的N即被视为缺乏。喀麦隆的油棕也有N缺乏的报道36,N缺乏主要影响叶片的生成、大小、颜色和净同化速率17。N供应不足时,油棕生长受抑,且随树龄增长而日益加剧17。
Phosphorus in all pinnae samples from Sites A and B were in the deficiency range for E. guineensis (Table 1). These P concentrations were lower than those reported in Indonesia, Malaysian and Nigerian E. guineensis leaves of 1500–1700 mg kg-17, 1210–1350 mg kg-114 and 1280 mg kg-114, respectively. The P concentration in leaves at Site C (1689 mg kg-1) was within the adequate range for E. guineensis and comparable to the value of 1700 mg kg-1 from E. guineensis also grown in Indonesia reported by Woittiez et al.7. The range of leaf P concentrations across the sites were comparable to those of New Zealand native species grown in low-fertility systems in nutrient-poor, non-fertilised soils37. This indicates the low nutrient status of the E. guineensis trees we sampled and is consistent with inadequate fertilisation. Sites A and B may have had low native P concentrations followed by insufficient capital and maintenance nutrients applied during production. Unlike N, P concentrations do not typically drop precipitously following site abandonment as P may bind to soil colloids and be retained in soils38. This indicates that P concentrations at Sites A and B were sub-optimal during production and may have been a contributing factor to low yields and subsequent site abandonment. Deficiencies of P in oil palm result in reduced growth rates with smaller fruit bunches, leaves and trunks, reducing yields from these trees17.
样地A和B所有羽片样品中的磷均处于E. guineensis的缺乏范围(表1)。这些P浓度低于印度尼西亚、马来西亚和尼日利亚E. guineensis叶片的报道值,分别为1500–1700 mg kg-17、1210–1350 mg kg-114和1280 mg kg-114。样地C叶片的P浓度(1689 mg kg-1)处于E. guineensis的适宜范围,与Woittiez et al.7报道的同样种植于印度尼西亚的E. guineensis的数值1700 mg kg-1相当。各样地叶片P浓度范围与生长于养分贫瘠、未施肥土壤的低肥力系统中的新西兰本土植物物种相当37。这表明我们所采样的E. guineensis植株养分状况较低,与施肥不足相符。样地A和B可能原本P浓度较低,加之生产期间基础养分和维持养分施用不足。与N不同,P可与土壤胶体结合并保留在土壤中,因此样地废弃后P浓度通常不会急剧下降38。这表明样地A和B在生产期间P浓度即处于次优水平,可能是导致产量低下和随后样地废弃的原因之一。油棕缺P会导致生长速率降低,果串、叶片和树干变小,从而降低产量17。
Rachis concentrations of K have been suggested as a more accurate indication of plant K status compared to pinnae concentrations as they provide a more accurate indication of fruit yield39. The K concentrations of the rachis samples range from 6204 mg kg-1 at Site B to 8969 mg kg-1 at Site A, indicating K deficiency (Table 1). Potassium deficiency is the most limiting nutrient factor affecting yield in oil palm production17,40,41. Like P, deficiencies of K in oil palm result in smaller fruit bunches as well as reduced number of fruit bunches per tree17. Insufficient K also leads to reduced disease resistance in oil palms17. Deficiency of this element has been attributed to inadequate K fertilisation of production soils which already have naturally low background levels7,36. Cost has been cited as a barrier to K fertilisation for Indonesian smallholders, as K fertilisers are not subsidised7. Concentrations of K in oil palm leaves from Indonesia and Malaysia have also been reported in deficient ranges of 6000–6300 mg kg-17 and 5700–7600 mg kg-114 respectively. Non-deficient levels of 8800 mg kg-1 were measured in Nigerian oil palm leaves14.
有研究认为,相比羽片浓度,叶轴中的K浓度能更准确地指示植物K营养状况,因为其对果实产量的指示更为准确39。叶轴样品的K浓度介于样地B的6204 mg kg-1至样地A的8969 mg kg-1之间,表明存在K缺乏(表1)。缺钾是影响油棕生产产量的最主要养分限制因子17,40,41。与P相似,油棕缺K会导致果串变小以及单株果串数减少17。K不足还会降低油棕的抗病性17。该元素的缺乏被归因于对本身背景水平即较低的生产土壤施用K肥不足7,36。由于钾肥不享受补贴,成本被认为是印度尼西亚小农户施用钾肥的障碍7。印度尼西亚和马来西亚油棕叶片的K浓度也有处于缺乏范围的报道,分别为6000–6300 mg kg-17和5700–7600 mg kg-114。尼日利亚油棕叶片中测得的K浓度为8800 mg kg-1,未处于缺乏水平14。
Among the three sites, 90% of pinnae samples from Site A, 71% of samples from Site B and 100% of samples from Site C were deficient in S. The S concentrations were comparable to those of Nigerian E. guineensis (1740 mg kg-1)14. Sulphur deficiency in oil palms has similar effects to N deficiency, i.e., stunted leaf growth and necrosis, as well as potential decreased resistance to Cercospora infection17. Boron was below the optimal range at Site C, and lower than reported concentrations for oil palm leaves also grown in North Sumatra (16.4–19.5 mg kg-1), which were expressing B deficiency symptoms42. Boron is the most significant TE for oil palm growth: with insufficient B, leaf development is severely affected and leaves become thin, short and brittle17. There is little information available on the role of Mo in oil palm growth17 and no studies reporting Mo concentration of E. guineensis leaves could be identified for comparison.
在三个样地中,样地A 90%的羽片样品、样地B 71%的样品和样地C 100%的样品缺乏S。S浓度与尼日利亚E. guineensis相当(1740 mg kg-1)14。油棕缺硫的影响与缺氮相似,即叶片生长受阻和坏死,并可能降低对Cercospora侵染的抗性17。样地C的B低于最适范围,且低于同样种植于北苏门答腊、表现出缺B症状的油棕叶片的报道浓度(16.4–19.5 mg kg-1)42。硼是对油棕生长最重要的微量元素:B不足时叶片发育受到严重影响,叶片变得薄、短且脆17。关于Mo在油棕生长中作用的资料很少17,且未能找到报道E. guineensis叶片Mo浓度的研究以供比较。
Magnesium, Fe, Cu and Zn in pinnae samples were within the adequate range for oil palm growth at all sites (Table 1). The Mg concentrations were comparable to those in leaves of E. guineensis grown in Indonesia and Nigeria of 2800–3000 mg kg-1 and 2330 mg kg-114, respectively. Zinc concentrations were comparable to leaf concentrations from Malaysian E. guineensis plants of ca. 15–28 mg kg-143. The Fe and Cu pinnae concentrations were within typical ranges contained in plant leaves12. Manganese was present in high concentrations in pinnae samples, however still within the range of concentrations likely to be present in plants44. Concentrations were significantly higher at Site B compared with Site A (Table 1). Toxicity thresholds for Mn are plant- and even cultivar-specific12, and no specific thresholds for oil palm have been identified. Considering differences between active and former production sites, the active site (C) was significantly higher in N and P than former sites (A and B) and significantly higher in Mo than Site B. This may be due to the Site C’s ongoing cultivation at the time of sampling, and thus more recent fertilisation.
所有样地羽片样品中的镁、Fe、Cu和Zn均处于油棕生长的适宜范围(表1)。Mg浓度与印度尼西亚和尼日利亚种植的E. guineensis叶片相当,分别为2800–3000 mg kg-1和2330 mg kg-114。锌浓度与马来西亚E. guineensis植株的叶片浓度(约15–28 mg kg-143)相当。羽片中Fe和Cu浓度处于植物叶片的典型范围内12。羽片样品中锰浓度较高,但仍处于植物中可能存在的浓度范围内44。样地B的浓度显著高于样地A(表1)。Mn的毒性阈值因植物甚至品种而异12,目前尚未确定油棕的具体阈值。就在产与原生产样地的差异而言,在产样地(C)的N和P显著高于原生产样地(A和B),Mo显著高于样地B。这可能是由于样地C在采样时仍在耕作,因而施肥时间较近。
Our leaf samples were collected from plantations with soils deficient in N, P, K and Mo23. Thus, it is unsurprising that plant concentrations of these essential elements are sub-optimal and likely to be limiting production, as plants source the majority of their nutrient requirements from bioavailable elements in soils through diffusion and mass flow12. These deficiencies are attributed to the conversion of acidic, low-fertility forest soils to production without the full amount of necessary inputs of both capital and maintenance nutrients4,5. As E. guineensis producers in Indonesia rely heavily on subsidised fertilisers, these deficiencies—particularly K for which no subsidised fertilisers are available—are commonplace, particularly in smallholder plantations7,40.
我们的叶片样品采自土壤缺乏N、P、K和Mo的种植园23。由于植物所需养分大部分通过扩散和质流从土壤中的生物有效态元素获取12,因此植物中这些必需元素浓度处于次优水平并可能限制生产也就不足为奇。这些缺乏被归因于酸性低肥力森林土壤在转为生产用地时,未足量投入所需的基础养分和维持养分4,5。由于印度尼西亚E. guineensis生产者严重依赖补贴化肥,这些缺乏(尤其是无补贴化肥可用的K)十分普遍,在小农户种植园中尤为如此7,40。
Non‑essential trace elements非必需微量元素
Most non-essential elements were present in concentrations less than the average concentrations for terrestrial plants (Table 2). The low concentrations of Cr (1.7–4.7 mg kg-1 in pinnae, 1.1–10 mg kg-1 in rachides) and Ti (1.5–1.8 mg kg-1 in pinnae, 0.60–0.87 mg kg-1 in rachides) indicate that the non-essential elements present in E. guineensis leaves were not a result of soil contamination of leaves. While Ti, Cr, Ni and Hg were present above average terrestrial plant concentrations45, they were below toxicity thresholds for leaf tissues15.
大多数非必需元素的浓度低于陆生植物的平均浓度(表2)。Cr(羽片中1.7–4.7 mg kg-1,叶轴中1.1–10 mg kg-1)和Ti(羽片中1.5–1.8 mg kg-1,叶轴中0.60–0.87 mg kg-1)浓度较低,表明E. guineensis叶片中的非必需元素并非源自叶片的土壤污染。虽然Ti、Cr、Ni和Hg高于陆生植物平均浓度45,但均低于叶片组织的毒性阈值15。
Mean concentrations of Na and Si were higher in rachides (170–192 mg kg-1 and 188–291 mg kg-1, respectively) compared with pinnae (54–116 mg kg-1 and 1.3 mg kg-1, respectively). Cadmium concentrations (0.020–0.027 mg kg-1 in pinnae, 0.010–0.014 mg kg-1 in rachides) were lower than those reported from Malaysian E. guineensis leaves (0.18–0.38 mg kg-1)43. Silver and Au were present in leaf tissues in concentrations < 0.1 mg kg-1 and pose no toxicity risks46.
叶轴中Na和Si的平均浓度(分别为170–192 mg kg-1和188–291 mg kg-1)高于羽片(分别为54–116 mg kg-1和1.3 mg kg-1)。镉浓度(羽片中0.020–0.027 mg kg-1,叶轴中0.010–0.014 mg kg-1)低于马来西亚E. guineensis叶片的报道值(0.18–0.38 mg kg-1)43。叶片组织中银和Au的浓度 < 0.1 mg kg-1,不构成毒性风险46。
| Site样点 | A (n = 10) | B (n = 7) | C (pinnae n = 2, rachides n = 1)C(羽片 n = 2,叶轴 n = 1) | Land plants average *陆生植物平均值* | Excessive/toxic to plants+对植物过量/有毒+ | |
|---|---|---|---|---|---|---|
| Na | 116(15)a | 111(21)a | 54(20)a | 1200 | – | |
| Al | 46(5.4)a | 44(4.5)a | 30(9.2)a | 500 | – | |
| Si | 1.3(0.019)a | 1.3(0.014)a | 1.3(0.035)a | 200 | – | |
| Ti | 1.8(0.18)a | 1.6(0.20)a | 1.5(0.20)a | 1 | 50–200 | |
| Cr | 4.2(0.92)a | 4.7(1.1)a | 1.7(0.52)a | 0.23 | 5–30 | |
| Co | 0.071(0.010)a | 0.093(0.020)a | 0.04(< 0.01)a | 0.5 | 15–50 | |
| Ni | 3.6(0.51)b | 5.8(1.0)b | 1.1(0.080)a | 3 | 10–100 | |
| As | 0.030(< 0.01)a | 0.031(< 0.01)a | 0.025(< 0.01)a | 0.2 | 5–20 | |
| Pinnae | Sr | 16(2.7)a | 9.7(0.85)a | 17(0.90)a | 26 | – |
| Ag | < 0.01a | < 0.01a | < 0.01a | 0.06 | – | |
| Cd | 0.027(< 0.01)a | 0.023(< 0.01)a | 0.020(< 0.01)a | 0.6 | 5–30 | |
| Te | < 0.01a | < 0.01a | 0.29(0.29)b | – | – | |
| Cs | 0.18(0.030)a | 0.25(0.035)ab | 0.41(0.045)b | 0.2 | – | |
| Ce | 0.22(0.048)a | 0.39(0.061)a | 0.85(0.26)b | – | – | |
| Au | < 0.01a | < 0.01a | < 0.01a | 0.002 | – | |
| Hg | 0.045(< 0.01)a | 0.044(< 0.01)a | 0.052(0.015)a | 0.015 | 1–3 | |
| Pb | 0.64(0.060)a | 0.76(0.12)a | 0.62(0.15)a | 2.7 | 30–300 | |
| Na | 173(19)a | 170(14)a | 192a | 1200 | – | |
| Al | 18(2.7)a | 24(3.6)a | 13a | 500 | – | |
| Si | 273(28)a | 291(29)a | 188a | 200 | – | |
| Ti | 0.60(0.063)a | 0.87(0.11)a | 0.60a | 1 | – | |
| Cr | 10(3.6)a | 8.8(2.1)a | 1.1a | 0.23 | – | |
| Co | 0.134(0.040)a | 0.14(0.030)a | 0.020a | 0.5 | – | |
| Ni | 5.3(1.6)a | 5.5(1.2)a | 0.50a | 3 | – | |
| As | < 0.01)a | < 0.01a | < 0.01a | 0.2 | – | |
| Rachides | Sr | 11(1.2)a | 6.9(0.86)b | 6.6ab | 26 | – |
| Ag | < 0.01a | < 0.01a | < 0.01a | 0.06 | – | |
| Cd | 0.014(< 0.01)a | 0.010(< 0.01)a | 0.010a | 0.6 | – | |
| Te | < 0.01a | < 0.01a | < 0.01a | – | – | |
| Cs | 0.092(0.020)a | 0.18(0.020)b | 0.74c | 0.2 | – | |
| Ce | 0.060(0.010)a | 0.090(0.020)a | 0.07a | – | – | |
| Au | < 0.01a | < 0.01a | < 0.01a | 0.002 | – | |
| Hg | < 0.01a | < 0.01a | < 0.01a | 0.015 | – | |
| Pb | 0.27(0.051)a | 0.35(0.080)a | 0.080a | 2.7 | – |
The pinnae concentrations of Te at Site C (0.29 mg kg-1) were significantly higher than at Sites A and B, and higher than those reported in Angiosperm leaves of 0.017 mg kg-147. Cerium was also significantly higher in pinnae from Site C compared to Sites A and B. There is a scarcity of data on Te and Ce in plants with which to compare our results. Pinnae from Site C contained significantly higher concentrations of Cs than Site A, while rachides from Site C were significantly higher in Cs than Sites A and B. Caesium concentrations in pinnae at Sites B and C (0.25 and 0.41 mg kg-1, respectively) and rachides at Site C (0.74 mg kg-1) were higher than average plant concentrations of 0.2 mg kg-145. The higher Te, Cs and Ce at Site C may be due to current production, as these TEs may be present in agrichemicals which were being used at the site at the time of sampling.
样地C羽片中的Te浓度(0.29 mg kg-1)显著高于样地A和B,且高于被子植物叶片的报道值0.017 mg kg-147。样地C羽片中的铈也显著高于样地A和B。关于植物中Te和Ce的数据稀少,难以与我们的结果进行比较。样地C羽片中的Cs浓度显著高于样地A,而样地C叶轴中的Cs显著高于样地A和B。样地B和C羽片中的铯浓度(分别为0.25和0.41 mg kg-1)以及样地C叶轴中的铯浓度(0.74 mg kg-1)高于植物平均浓度0.2 mg kg-145。样地C中较高的Te、Cs和Ce可能与当前生产有关,因为这些微量元素可能存在于采样时该样地正在使用的农用化学品中。
Elements in E. guineensis endosperms and mesocarpsE. guineensis胚乳和中果皮中的元素
Essential elements必需元素
The essential elements in the endosperm tissues (Table 3) were comparable to those in Malaysian and Nigerian E. guineensis endosperms, except for Mg and Fe which were both lower in our samples43,48,49. Endosperm tissues contained the highest P and Cu concentrations of all plant materials analysed. Mesocarp tissues tended to contain the lowest concentrations of most elements, particularly essential plant elements, of all plant materials analysed.
胚乳组织中的必需元素(表3)与马来西亚和尼日利亚E. guineensis胚乳相当,但Mg和Fe在我们的样品中均较低43,48,49。在所分析的全部植物材料中,胚乳组织的P和Cu浓度最高。在所分析的全部植物材料中,中果皮组织中大多数元素(尤其是植物必需元素)的浓度往往最低。
Phosphorus and K in endosperm samples ranged from 3125–3827 mg kg-1 and 4870–5045 mg kg-1, respectively, within concentration ranges reported in Nigerian endosperms: 2600–4700 and 2770–6600 mg kg-1, respectively49. These concentrations were lower than those in Malaysian endosperms: 6520–6950 and 6930–7510 mg kg-1, respectively48. The concentrations of Mn in endosperm samples (136–285 mg kg-1) overlapped with the range reported in Malaysian endosperms (82–145 mg kg-1)49 but were lower than Mn concentrations reported in Nigerian samples of 410–610 mg kg-148. Our Cu and Zn concentrations in endosperms tissue (16–17 and 24–27 mg kg-1, respectively) were similar to the ranges present in Malaysian endosperms of 16–18 and 25–36 mg kg-1, respectively49 and lower than those of Nigerian endosperm tissue48. Magnesium and Fe concentrations in our analysed samples were lower than those from Malaysia (2050–3060 mg kg-1 Mg and 43–52 mg kg-1 Fe)48 and Nigeria (2250–5540 mg kg-1 Mg and 110–220 mg kg-1 Fe)49. No data could be identified for comparison on concentrations of C, N, S, B or Mo in E. guineensis endosperm tissue. There were only two significant differences in concentrations of essential elements in endosperm tissues between sites: Site A was significantly higher in B than site B, while Site B was significantly higher in Mo than Site C.
胚乳样品中的磷和K分别为3125–3827 mg kg-1和4870–5045 mg kg-1,处于尼日利亚胚乳的报道浓度范围内(分别为2600–4700和2770–6600 mg kg-1)49。这些浓度低于马来西亚胚乳(分别为6520–6950和6930–7510 mg kg-1)48。胚乳样品中的Mn浓度(136–285 mg kg-1)与马来西亚胚乳的报道范围(82–145 mg kg-1)49部分重叠,但低于尼日利亚样品的报道Mn浓度410–610 mg kg-148。我们测得胚乳组织中的Cu和Zn浓度(分别为16–17和24–27 mg kg-1)与马来西亚胚乳的范围(分别为16–18和25–36 mg kg-1)49相近,且低于尼日利亚胚乳组织48。所分析样品中的镁和Fe浓度低于马来西亚(Mg 2050–3060 mg kg-1,Fe 43–52 mg kg-1)48和尼日利亚(Mg 2250–5540 mg kg-1,Fe 110–220 mg kg-1)49的样品。未能找到E. guineensis胚乳组织中C、N、S、B或Mo浓度的数据以供比较。各样地间胚乳组织必需元素浓度仅有两处显著差异:样地A的B显著高于样地B,而样地B的Mo显著高于样地C。
| Site样点 | A (n = 8) | B (n = 7) | C (n = 3) | ||
|---|---|---|---|---|---|
| C (%) | 61(0.37)a | 62(0.41)a | 60(1.0)a | ||
| N (%) | 1.4(0.10)a | 1.3(0.12)a | 1.3(0.19)a | ||
| Macro-elements | P | 3618(131)a | 3827(189)a | 3125(16)a | |
| K | 4870(109)a | 5045(326)a | 4932(414)a | ||
| S | 1665(79)a | 1554(89)a | 1456(114)a | ||
| Endoserm | Mg | 1958(76)a | 1937(115)a | 1574(105)a | |
| p | B | 67(7.8)b | 37(3.8)a | 52(6.4)ab | |
| Mn | 136(18)a | 285(69)a | 157(20)a | ||
| Milt | Fe | 32(1.3)a | 37(2.7)a | 37(5.5)a | |
| cro-eemens | Cu | 17(0.73)a | 16(0.8)a | 17(1.7)a | |
| Zn | 24(1.4)a | 27(2.3)a | 26(2.6)a | ||
| Mo | 0.24(0.033)ab | 0.34(0.060)b | 0.1(0.019)a | ||
| C (%) | 66(1.7)a | 70(1.0)a | 64(4.4)a | ||
| N (%) | 0.29(0.02)a | 0.31(0.044)a | 0.42(0.035)a | ||
| l | P | 513(53)a | 484(25)a | 849(85)b | |
| Macro-eements | K | 4487(605)ab | 3044(192)a | 6876(1894)b | |
| S | 981(92)a | 815(29)a | 994(74)a | ||
| Mg | 1166(180)a | 803(84)a | 1516(206)a | ||
| Mesocarp | B | 51(4.4)a | 45(4.0)a | 57(11)a | |
| Mn | 5.6(0.70)a | 10(2.4)a | 14(5.5)a | ||
| Fe | 35(2.9)b | 25(1.8)a | 33(6.3)ab | ||
| Micro-elements | Cu | 15(1.4)a | 14(1.0)a | 14(0.80)a | |
| Zn | 4(0.47)a | 3.7(0.443)a | 8.2(1.1)b | ||
| Mo | 0.056(0.011)a | 0.063(0.016)a | 0.033(< 0.01)a |
The low concentrations in mesocarp tissues (Table 3) are typical of E. guineensis: as fruit ripens, essential elements in the mesocarp decrease due to dilution by growth or translocation into the endosperm14. Our samples were ripe when collected, and the concentration ranges of N, P, K and Mg—0.29–0.42%, 484–849 mg kg-1, 3044–6876 mg kg-1, 803–1516 mg kg-1, respectively—are comparable to those of ripe mesocarp: 0.33–0.41%, 440–530 mg kg-1, 2900–3700 mg kg-1, 1300–1500 mg kg-1, respectively50. Of the essential elements analysed, N, P, Mg, S Mn, Cu, Zn, and Mo were significantly higher in endosperms compared to mesocarps.
中果皮组织中的低浓度(表3)是E. guineensis的典型特征:随着果实成熟,中果皮中的必需元素因生长稀释或向胚乳转运而减少14。我们的样品采集时已成熟,其N、P、K和Mg的浓度范围(分别为0.29–0.42%、484–849 mg kg-1、3044–6876 mg kg-1、803–1516 mg kg-1)与成熟中果皮(分别为0.33–0.41%、440–530 mg kg-1、2900–3700 mg kg-1、1300–1500 mg kg-1)相当50。在所分析的必需元素中,胚乳的N、P、Mg、S、Mn、Cu、Zn和Mo显著高于中果皮。
Non‑essential trace elements非必需微量元素
Excluding Na, Al, Si, Cr, Ni and Sr, all non-essential elements in E. guineensis endosperms and mesocarps were < 1.0 mg kg-1 (Table 4). Non-essential elements posed no toxicity risks for manufactured products. As palm oil is expressed or extracted from the mesocarp, the low concentrations in this plant material indicates that TE concentrations in palm oil are likely to be low and of no concern regarding food safety standards, unless it is contaminated during the extraction process. As with leaf concentrations, Cs was significantly higher in mesocarps from Site C. Other than this, there were no significant differences in mesocarps between sites. Low elemental concentrations are typical of endosperm tissue, as to reach this location of the plant elements must be carried by phloem transport and cross the placenta51. As with leaves, Ni was significantly lower in mesocarp tissue from Site C site compared with Sites A and B. Chromium was also significantly higher in mesocarps from Site A compared to Site B.
除Na、Al、Si、Cr、Ni和Sr外,E. guineensis胚乳和中果皮中所有非必需元素均 < 1.0 mg kg-1(表4)。非必需元素对加工产品不构成毒性风险。由于棕榈油是从中果皮中压榨或提取的,该植物材料中的低浓度表明,除非在提取过程中受到污染,棕榈油中的微量元素浓度可能较低,不会引起食品安全标准方面的担忧。与叶片浓度一样,样地C中果皮中的Cs显著较高。除此之外,各样地中果皮之间无显著差异。元素浓度低是胚乳组织的典型特征,因为元素须经韧皮部运输并穿过胎座方能到达植物的这一部位51。与叶片一样,样地C中果皮组织中的Ni显著低于样地A和B。样地A中果皮中的铬也显著高于样地B。
Mean Na in the endosperm samples ranged from 112–223 mg kg-1, within the range of 80–240 mg kg-1 from Malaysian kernels49 and below the range of 610–1200 mg kg-1 from Nigerian kernels48. Cadmium in our endosperm samples (0.02–0.03 mg kg-1) was lower than in samples from Malaysia (0.09–0.31 mg kg-1)43, while Pb (0.02–0.03 mg kg-1) was comparable to the below-detection concentrations of ≤ 0.05 mg kg-1 reported in Nigerian kernels48.
胚乳样品中Na的平均值为112–223 mg kg-1,处于马来西亚果仁的范围80–240 mg kg-1之内49,并低于尼日利亚果仁的范围610–1200 mg kg-148。我们胚乳样品中的镉(0.02–0.03 mg kg-1)低于马来西亚样品(0.09–0.31 mg kg-1)43,而Pb(0.02–0.03 mg kg-1)与尼日利亚果仁中报道的低于检出限的浓度(≤ 0.05 mg kg-1)相当48。
| Site样点 | A (n = 8) | B (n = 7) | C (n = 3) | |
|---|---|---|---|---|
| Na | 223(33)a | 128(15)b | 112(24)ab | |
| Al | 31(5.2)a | 17(2.9)a | 27(4.9)a | |
| Si | 352(38)a | 303(38)a | 226(22)a | |
| Ti | 0.33(0.016)a | 0.39(0.051)a | 0.30(< 0.01)a | |
| Cr | 0.29(0.018)b | 0.19(0.027)a | 0.24(0.064)ab | |
| Co | 0.013(< 0.01)a | 0.014(< 0.01)a | 0.010(< 0.01)a | |
| Ni | 1.6(0.17)b | 2.2(0.35)b | 0.60(0.13)a | |
| As | < 0.01a | < 0.01a | < 0.01a | |
| Endosperm | Sr | 5.0(0.59)a | 4.6(0.32)a | 3.9(0.44)a |
| Ag | < 0.01a | < 0.01a | < 0.01a | |
| Cd | 0.018(< 0.01)a | 0.027(< 0.01)a | 0.017(< 0.01)a | |
| Te | < 0.01a | < 0.01a | < 0.01a | |
| Cs | 0.068(0.015)a | 0.094(0.023)a | 0.13(0.022)a | |
| Ce | 0.16(0.028)a | 0.080(0.014)a | 0.14(0.023)a | |
| Au | < 0.01a | < 0.01a | < 0.01a | |
| Hg | < 0.01a | < 0.01a | < 0.01a | |
| Pb | 0.031(< 0.01)a | 0.021(< 0.01)a | 0.027(< 0.01)a | |
| Na | 213(29)a | 164(9.4)a | 180(27)a | |
| Al | 35(6.3)a | 28(3.1)a | 31(8.6)a | |
| Si | 328(22)a | 320(12)a | 313(38)a | |
| Ti | 0.50(0.17)a | 0.40(0.044)a | 0.30(0.12)a | |
| Cr | 3.8(0.28)a | 2.6(0.39)a | 4.0(1.0)a | |
| Co | 0.070(< 0.01)a | 0.066(0.010)a | 0.060(0.012)a | |
| Ni | 2.1(0.15)a | 1.6(0.18)a | 2.0(0.36)a | |
| As | < 0.01a | < 0.01a | < 0.01a | |
| Mesocarp | Sr | 4.5(0.64)a | 4.4(0.47)a | 6.3(1.3)a |
| Ag | < 0.01a | < 0.01a | 0.010(< 0.01)a | |
| Cd | 0.014(< 0.01)a | 0.011(< 0.01)a | 0.010(< 0.01)a | |
| Te | < 0.01a | < 0.01a | < 0.01a | |
| Cs | 0.24(0.074)a | 0.28(0.071)a | 0.73(0.082)b | |
| Ce | 0.13(0.014)a | 0.11(0.014)a | 0.13(0.040)a | |
| Au | < 0.01a | < 0.01a | < 0.01a | |
| Hg | < 0.01a | < 0.01a | < 0.01a | |
| Pb | 0.053(0.014)a | 0.047(0.011)a | 0.060(0.015)a |
| Site A样点A | Site B样点B | Site C样点C | |||||||
|---|---|---|---|---|---|---|---|---|---|
| Pinnae | Endosperm | Mesocarp | Pinnae | Endosperm | Mesocarp | Pinnae | Endosperm | Mesocarp | |
| Cu | 0.31 | 0.89 | 0.79 | 0.16 | 0.42 | 0.37 | 1.4 | 3.0 | 2.5 |
| Zn | 0.27 | 0.26 | 0.044 | 0.26 | 0.30 | 0.041 | 0.31 | 0.35 | 0.11 |
| As | 0.0079 | < 0.0026 | < 0.0026 | 0.0072 | < 0.0026 | < 0.0023 | 0.0027 | < 0.0011 | < 0.0011 |
| Sr | 0.67 | 0.21 | 0.19 | 0.69 | 0.33 | 0.31 | 0.35 | 0.81 | 0.13 |
| Cd | 0.19 | 0.13 | 0.10 | 0.26 | 0.31 | 0.13 | 0.24 | 0.20 | 0.12 |
| Pb | 0.040 | 0.0019 | 0.0033 | 0.045 | 0.0012 | 0.0028 | 0.022 | 0.0010 | 0.0021 |
Bioaccumulation coefficients生物累积系数
Most BACs for TEs in E. guineensis at the sites sampled were < 0.5 (Table 5). A BAC of ≥ 1 indicates that a plant may take up higher than typical concentrations of a TE from soil31. These results are consistent with low BACs of most non-essential TEs measured in other studies52,53 except for Sr, for which no BACs could be identified from literature.
所采样地E. guineensis中大多数微量元素的BACs < 0.5(表5)。BAC ≥ 1表明植物可能从土壤中吸收高于一般水平的某种微量元素31。这些结果与其他研究中测得的大多数非必需微量元素BACs较低的结果一致52,53,但Sr除外,文献中未能找到其BACs。
The BAC of Cu in all plant tissues at Site C was > 1, indicating E. guineensis here contained high concentrations of Cu relative to the soils at this site. This may have been due to direct application of Cu-containing spray residues onto plant tissues, as this site was still under active management, however, this is unlikely as endosperm and mesocarp tissue had higher BACs relative to pinnae. Leaf tissues typically receive foliar spray applications while internal fruit tissues do not, therefore if this were the reason for the high BACs at this site, it is likely that endosperm and mesocarp BACs would be lower than that of pinnae tissues. While it is possible that Cu may be translocated from the leaf to the fruit following direct contamination of leaves with Cu spray, the higher BACs of fruit tissue relative to leaf tissue indicate that Cu was likely entering plants via root uptake from soil solution and was highly phloem-mobile. This is supported by the BACs for Cu in fruit tissues at Site A (0.89 and 0.79 for endosperm and mesocarp, respectively), which were higher than the pinnae BAC at this site. The high BAC of Cu in E. guineensis fruit tissues may result in high Cu concentrations in plant products, including oil and PKE, if production soils contain excessive Cu concentrations. This may present risks to human and animal health if food and fodder safety standards, respectively, for Cu are exceeded.
样地C所有植物组织中Cu的BAC均 > 1,表明此处的E. guineensis相对于该样地土壤含有较高浓度的Cu。这可能是由于含Cu喷雾残留物直接施用于植物组织所致,因为该样地仍处于积极管理之中;然而这种可能性不大,因为胚乳和中果皮组织的BACs高于羽片。叶片组织通常接受叶面喷施,而果实内部组织则不会,因此若此为该样地BACs较高的原因,胚乳和中果皮的BACs可能会低于羽片组织。虽然叶片受Cu喷雾直接污染后Cu有可能从叶片转运至果实,但果实组织BACs高于叶片组织表明,Cu很可能是经根系从土壤溶液吸收进入植物,且在韧皮部中具有高度移动性。样地A果实组织中Cu的BACs(胚乳和中果皮分别为0.89和0.79)高于该样地羽片的BAC,也支持了这一点。若生产土壤中Cu浓度过高,E. guineensis果实组织中Cu的高BAC可能导致植物产品(包括油和棕榈仁粕(PKE))中Cu浓度较高。若分别超出食品和饲料安全标准中Cu的限值,则可能对人类和动物健康构成风险。
The BAC of Sr in pinnae at both Sites A and B (0.67 and 0.69, respectively) indicated that Sr was likely entering plant tissues E. guineensis at these sites via soils. The BAC of Sr at Site C (0.81) also indicated that Sr maybe phloem mobile and easily transported to fruit tissues. There is little published information on Sr BACs or transport in plants with which to compare these results.
样地A和B羽片中Sr的BAC(分别为0.67和0.69)表明,这些样地的Sr很可能经土壤进入E. guineensis植物组织。样地C中Sr的BAC(0.81)也表明Sr可能具有韧皮部移动性,易于运输至果实组织。关于植物中Sr的BACs或运输的已发表资料很少,难以与这些结果进行比较。
As E. guineensis is cultivated in plantations with differing management styles, including smallholder, corporate- and government-owned54, the determination of BACs for fertiliser contaminants in E. guineensis grown under a range of conditions with differing agrichemical input rates may be of benefit to this production systems. This research may develop strategies to limit the transfer of contaminants to plants and products if increased fertiliser applications were used to correct nutrient deficiencies.
由于E. guineensis种植园的管理方式各不相同,包括小农户、企业和政府所有54,因此测定在不同条件、不同农用化学品投入水平下种植的E. guineensis中肥料污染物的BACs可能对该生产系统有益。若为纠正养分缺乏而增加施肥量,此类研究可有助于制定限制污染物向植物及产品迁移的策略。
Elements in palm oil棕榈油中的元素
Unlike TEs, plant oils are not transported by xylem or phloem from leaves to fruit tissue but are synthesised from sugars in situ18. Most TEs occur as hydrophilic metal complexes in plants, partitioning away from oils in plant tissues55. As such, high TE concentrations in vegetable oils are not common. Elemental concentrations in refined palm oil were lower than food safety standards and posed no risk of elemental toxicity. However, this study did not analyse pesticide residues which may be present in oils. No elements in the oil we analysed exceeded tolerable upper limits or maximum dietary reference intakes (Table 6). This is consistent with other studies addressing the elemental composition of plant-derived oils, in which TEs were found either below detection limits or in concentrations ≤ 1.0 mg kg-156,57.
与微量元素不同,植物油并非经木质部或韧皮部从叶片运输至果实组织,而是在原位由糖合成的18。大多数微量元素在植物中以亲水性金属络合物的形式存在,在植物组织中分配于油脂之外55。因此,植物油中微量元素浓度高的情况并不常见。精炼棕榈油中的元素浓度低于食品安全标准,不存在元素毒性风险。但本研究未分析油中可能存在的农药残留。我们所分析的油中没有任何元素超过可耐受最高摄入量或膳食参考摄入量上限(表6)。这与其他关于植物源油脂元素组成的研究一致,这些研究发现微量元素或低于检出限,或浓度 ≤ 1.0 mg kg-156,57。
The following elements were present in our analysed palm oil at concentrations comparable to or less than concentrations in palm oils from previous studies: Mg, P, K, Ca, Cr, Mn, Fe, Co, Ni, Cu, Zn, As, Cd, Hg and Pb (Table 6). Concentrations of Na and Al in our palm oil samples were higher than previously reported. The mean concentration of Na in our samples was 1198 mg kg-1. This is higher than reported levels in Nigerian palm oils of 30 mg kg-158 and 115–533 mg kg-159, however, would not result in consumption beyond the tolerable upper limit of 2300 mg Na day-1. The mean concentration of Al in our palm oil samples (159 mg kg-1) was also higher than those previously reported in Nigerian palm oil by Obi et al.58 (31 mg kg-1) and Asemave et al.60 (1.9 mg kg-1), however below concentrations which would surpass its tolerable weekly intake of 1 mg kg-1 bw wk-1, assuming an average body weight of 70 kg61 and an average daily palm oil intake of 37.1 g62. For people weighing < 41 kg, exceedance of the tolerable weekly intake may occur if they are consuming ≤ 37.1 g of palm oil per day, the average vegetable oil consumption in China—a major importer of palm oil. High Al and Na in plant derived products are usually attributed to soil or dust contamination of plant materials (e.g., during harvesting)63, however as these elements were found in the oil they may also come from processing. Other potential reasons for higher concentrations of these elements in the samples analysed include the use of saline washdown water in mills. The high Al concentrations in palm oil are supported by the mean Al concentrations in mesocarp samples (28–35 mg kg-1). Unlike most other TEs, Al may form hydrophobic organic complexes in plants which are phloem mobile, thereby partitioning into palm oil in the mesocarp64.
我们所分析的棕榈油中以下元素的浓度与以往研究中棕榈油的浓度相当或更低:Mg、P、K、Ca、Cr、Mn、Fe、Co、Ni、Cu、Zn、As、Cd、Hg和Pb(表6)。我们棕榈油样品中Na和Al的浓度高于以往报道。样品中Na的平均浓度为1198 mg kg-1。这高于尼日利亚棕榈油的报道水平30 mg kg-158和115–533 mg kg-159,但不会导致摄入量超过可耐受最高摄入量2300 mg Na day-1。我们棕榈油样品中Al的平均浓度(159 mg kg-1)也高于Obi et al.58(31 mg kg-1)和Asemave et al.60(1.9 mg kg-1)此前报道的尼日利亚棕榈油,但在假设平均体重为70 kg61、日均棕榈油摄入量为37.1 g62的情况下,低于会超过其每周可耐受摄入量1 mg kg-1 bw wk-1的浓度。对于体重 < 41 kg的人群,若每天摄入 ≤ 37.1 g棕榈油(中国(棕榈油主要进口国)的平均植物油消费量),则可能超过每周可耐受摄入量。植物源产品中Al和Na含量高通常归因于植物材料受到土壤或粉尘污染(例如在收获期间)63,但由于这些元素存在于油中,它们也可能来自加工过程。所分析样品中这些元素浓度较高的其他可能原因包括油厂使用含盐冲洗水。中果皮样品中的平均Al浓度(28–35 mg kg-1)也佐证了棕榈油中Al浓度较高。与大多数其他微量元素不同,Al可在植物中形成具有韧皮部移动性的疏水性有机络合物,从而在中果皮中分配进入棕榈油64。
3Conclusions结论
The E. guineensis plant materials from North Sumatra, Indonesia, were deficient in essential elements including N, P, K and Mo, likely reducing palm oil yields from these sites. This is consistent with our hypotheses that E. guineensis leaves will show nutrient deficiencies, however, Mg was not deficient in leaf tissue as we had hypothesised. Leaf tissue from all sites was deficient in K, indicating that K may have been a yield-limiting factor potentially leading to the abandonment of production at two of the sites sampled. There is clear evidence that element deficiencies contribute to site abandonment. Leaf tissues showed no sign of elevated Cu, Zn, As and Pb, which falsified our hypothesis that leaves may contain elevated levels of TEs. Copper, however, had BACs > 1, indicating either elevated plant uptake or surface contamination from Cu-containing agrichemicals. This may result in E. guineensis-based products that exceed food and fodder safety standards if plants are grown on soils with excessive Cu concentrations. Palm oil generally contained low concentrations of TEs which were not likely to pose any toxicity risks. This was consistent with our hypothesis and with plant physiology considering trace elements often occur in plants as metal complexes which partition away from the oil phase. Aluminium and Na were present in palm oil at higher concentrations than had been previously reported in other studies, however, were not in breach of food safety standards. Future work could assess the bioaccumulation coefficients of TEs in E. guineensis under a range of conditions to determine whether plant tissues or oils may exceed toxicity thresholds or food safety standards with large fertiliser applications. This could be achieved in a dose–response pot trial. This would inform reasonable limits for fertiliser applications and contaminants to limit the transfer of TEs to plants and products in palm oil production systems.
来自印度尼西亚北苏门答腊的E. guineensis植物材料缺乏N、P、K和Mo等必需元素,可能降低了这些样地的棕榈油产量。这与我们关于E. guineensis叶片将表现出养分缺乏的假设一致,但叶片组织中Mg并未如我们假设的那样缺乏。所有样地的叶片组织均缺K,表明K可能是产量限制因子,并可能导致所采样的两个样地停止生产。有明确证据表明元素缺乏是导致样地废弃的原因之一。叶片组织未显示Cu、Zn、As和Pb升高的迹象,从而否定了叶片可能含有高水平微量元素的假设。然而,Cu的BACs > 1,表明植物吸收增加或受到含Cu农用化学品的表面污染。若植物种植于Cu浓度过高的土壤上,这可能导致以E. guineensis为原料的产品超出食品和饲料安全标准。棕榈油中微量元素浓度总体较低,不太可能构成任何毒性风险。这与我们的假设以及植物生理学相符,因为微量元素在植物中常以金属络合物形式存在,分配于油相之外。棕榈油中铝和Na的浓度高于其他研究以往的报道,但未超出食品安全标准。今后的工作可评估不同条件下微量元素在E. guineensis中的生物累积系数,以确定在大量施肥时植物组织或油脂是否会超过毒性阈值或食品安全标准。这可以通过剂量–效应盆栽试验实现。由此可为确定肥料施用量和污染物的合理限值提供依据,以限制棕榈油生产系统中微量元素向植物及产品的迁移。
| Element元素 | Mean (mg kg-1) (n = 10)平均值(mg kg-1)(n = 10) | Maximum consumed quantity (mg day-1) *最大摄入量(mg day-1)* | Tolerable upper limit (mg day-1)+可耐受最高摄入量(mg day-1)+ | Total ranges reported in other studies (mg kg-1)其他研究报道的 总范围(mg kg-1) |
|---|---|---|---|---|
| Na | 1198(155) | 44 | 2300 | 30–533ab |
| Mg | 3.1(0.41) | 0.12 | 350 | 0.02–192cabd |
| Al | 159(8.5) | 0.59 (mg kg-1bw wk-1)† | 1 (mg kg-1bw wk-1)† | 1.9–31ae |
| P | 3.5(0.077) | 0.13 | 4000 | 8–47f |
| S | 60(3.9) | 2.2 | – | – |
| K | 155(11) | 5.8 | 4500–4700‡ | 0.39–165bd |
| Ca | 51(2.8) | 1.9 | 2500 | 0.34–867cabd |
| Cr | 0.080(0.019) | < 0.01 | 0.02–0.04‡ | 0.02–2.3beg |
| Mn | 0.25(0.049) | < 0.01 | 11 | 0.24–12abh |
| Fe | 2.6(1.3) | 0.096 | 45 | 0.12–232cfbdeh |
| Co | 0.019(< 0.01) | < 0.01 | – | 0.00–0.06h |
| Ni | 0.031(0.010) | < 0.01 | 1 | 0.00–0.81bgh |
| Cu | 0.048(0.018) | < 0.01 | 10 | 0.00–2.1cfabeh |
| Zn | < 0.01 | < 0.01 | 40 | 0.05–15bdh |
| As | 0.014(< 0.01) | < 0.01 | – | ≤ 0.03gij |
| Sr | 0.22(< 0.01) | < 0.01 | – | – |
| Zr | 1.4(0.096) | 0.052 | – | – |
| Mo | 0.021(0) | < 0.01 | 2 | – |
| Ag | < 0.01 | < 0.01 | – | – |
| Cd | 0.015(< 0.01) | < 0.0001 (mg kg-1bw wk-1)† | 0.007 (mg kg-1bw wk-1)† | 0.02–0.09beg |
| Te | 0.010(< 0.01) | < 0.01 | – | – |
| Au | < 0.01 | < 0.01 | – | – |
| Hg | < 0.01 | < 0.0001 (mg kg-1bw wk-1)† | 0.0016 (mg kg-1bw wk-1)† | 0.00–0.06g |
| Pb | 0.075(0.012) | < 0.0001 (mg kg-1bw wk-1)† | 0.025 (mg kg-1bw wk−1)† | ≤ 0.07cfbeg |
4Data availability数据可用性
The data that support the findings of this study are openly available at www. kiwis cience. com/ Data/ Thomp son- Morri son- Plant Paper Data. xlsx.
支持本研究结果的数据可在www. kiwis cience. com/ Data/ Thomp son- Morri son- Plant Paper Data. xlsx公开获取。
Received: 7 July 2022; Accepted: 20 December 2023收稿日期:2022年7月7日;录用日期:2023年12月20日
5References参考文献
1. Shahbandeh, M. (2022). Consumption of vegetable oils worldwide from 2013/14 to 2021/2022, by oil type. Statista. Retrieved 9th May, 2022, from https:// www. stati sta. com/ stati stics/ 263937/ veget able- oils- global- consu mption/
2. OEC. (2020). Palm oil. Retrieved 17th May, 2022, from https:// oec. world/ en/ profi le/ hs/ palm- oil#: ~: text= In% 202020% 2C% 20the% 20top% 20exp orter s,and% 20Spa in% 20(% 241. 25B).
3. Vijay, V., Pimm, S. L., Jenkins, C. N. & Smith, S. J. The impacts of oil palm on recent deforestation and biodiversity loss. PLoS ONE 11(7), e0159668. https:// doi. org/ 10. 1371/ journ al. pone. 01596 68 (2016).
4. Foy, C. D. (1984). Physiological effects of hydrogen, aluminum, and manganese toxicities in acid soil. In F. Adams (Ed.), Agronomy monograph. https:// doi. org/ 10. 2134/ agron monog r12. 2ed. c2
5. Hartemink, A. E. (2002). Soil science in tropical and temperate regions—Some differences and similarities. In D. L. Sparks (Ed.), Advances in Agronomy (Vol. 77, pp. 269–292). Academic Press. https:// www. scien cedir ect. com/ scien ce/ artic le/ pii/ S0065 21130 27701 68 https:// doi. org/ 10. 1016/ S0065- 2113(02) 77016-8
6. Ng, S. K. Nutrition and nutrient management of oil palm—New thrust for the future perspective. In Potassium for sustainable crop production: International symposium on the role of potassium (eds Pasricha, N. S. & Bansal, S. K.) 415–429 (Potash Research Institute of India and International Potash Institute, 2002).
7. Woittiez, L. S., Slingerland, M. & Giller, K. E. Yield gaps in Indonesian smallholder plantations: Causes and solutions International Palm Oil Congress and Exhibition (Kuala Lumpur, 2015).
8. Chaney, R. L. Toxic element accumulation in soils and crops: protecting soil fertility and agricultural food chains. In Inorganic contaminants in the vadose zone (eds Bar-Yosef, B. et al.) 140–158 (Springer, 1989).
9. Aderungboye, F. O. Diseases of the oil palm. PANS 23(3), 305–326. https:// doi. org/ 10. 1080/ 09670 87770 94124 57 (1977).
10. MPOB. Chemical fertiliser Ganocare™ as preventive treatment in controlling ganoderma disease of oil palm (Malaysian Palm Oil Board TT No. 564) (2015). http:// palmo ilis. mpob. gov. my/ publi catio ns/ TOT/ TT564- Idris. pdf 11. Rys, G. J. A national cadmium management strategy for New Zealand agriculture. Cadmium Working Group (2011).
12. Marschner, H. Mineral nutrition of higher plants. Gulf Professional Publishing (1995).
13. Kabata-Pendias, A. & Mukherjee, A. B. Trace elements from soil to human (Springer Verlag, 2007). 14. Corley, R. H. V., & Tinker, P. B. H. The oil palm (5th ed.). Wiley (2015). https:// books. google. co. nz/ books? id= 71A1C AAAQB AJ 15. Kabata-Pendias, A., & Pendias, H. (2001). Trace elements in soil and plants (3rd ed.). CRC Press. 16. Hooda, P. Trace elements in soils (Wiley, 2010). 17. Von Uexküll, H. R., & Fairhurst, T. H. Fertilising for high yield and quality: The oil palm. International Potash Institute (1991). https:// www. ipipo tash. org/ uploa ds/ udocs/ ipi_ bulle tin_ 12_ ferti lizing_ for_ high_ yield_ and_ quali ty_ the_ oil_ palm. pdf 18. Salisbury, F. B., & Ross, C. W. Plant physiology (4th ed.). Wadsworth, Inc (1992). 19. Thompson-Morrison, H., Gaw, S. & Robinson, B. An assessment of trace element accumulation in palm oil production. Sustain‑ ability 14(8), 4553 (2022).
20. Gupta, M. Practical guide to vegetable oil processing. Elsevier Science (2017). https:// books. google. co. nz/ books? id= Ypp_ CwAAQ BAJ 21. Rossi, M., Gianazza, M., Alamprese, C., & Stanga, F. The role of bleaching clays and synthetic silica in palm oil physical refining. Food Chemistry, 82(2), 291–296 (2003). https:// doi. org/ 10. 1016/ S0308- 8146(02) 00551-4 22. Szydłowska-Czerniak, A., Trokowski, K., Karlovits, G., & Szłyk, E. Spectroscopic determination of metals in palm oils from different stages of the technological process. J. Agric. Food Chem. 61, 2276−2283 (2013). https:// doi. org/ 10. 1021/ jf305 094s 23. Thompson-Morrison, H., Ariantiningsih, F., Arief, S. M., Gaw, S. & Robinson, B. Nutrients and contaminants in soils of current and former oil palm production systems from Indonesia. Land 12(12), 2144. https:// doi. org/ 10. 3390/ land1 21221 44 (2023). 24. Encyclopedia Britannica. (2016). Acrisol. https:// www. brita nnica. com/ scien ce/ Acris ol
25. US EPA. Method 3051A (SW‑846): Microwave assisted acid digestion of sediments, sludges, soils, and oils, Revision 1. US EPA (2007). 26. Milestone. (n.d.). Digestion method for environmental samples. Milestone. 27. INCT. Polish certified reference material for multielement trace analysis: Oriental basma tobacco leaves (INCT‑OBTL‑5). Institute of Nuclear Chemistry and Technology (2010). 28. NIST. Certificate of analysis: Standard reference material 1573a tomato leaves. National Institute of Standards & Technology (1995). 29. NIST. Certificate of analysis: Standard reference material 1643f trace elements in water (2015). National Institute of Standards & Technology. 30. LECO. Instrument: CNS928 determination of carbon, nitrogen and sulfur in plant tissue. LECO corporation (2019). https:// eu. leco. com/ images/ Analy tical- Appli cation- Libra ry/ CNS928_ CNS_ PLANT_ TISSUE_ 203- 821- 592. pdf 31. Koleli, N., Demir, A., Kantar, C., Atag, G. A., Kusvuran, K., & Binzet, R. Heavy metal accumulation in serpentine flora of Mersin- Findikpinari (Turkey)—role of ethylenediamine tetraacetic acid in facilitating extraction of nickel. In K. R. Hakeem, M. Sabir, M. Öztürk, & A. R. Mermut (Eds.), Soil remediation and plants (pp. 629–659). Academic Press (2015). https:// www. scien cedir ect. com/ scien ce/ artic le/ pii/ B9780 12799 93710 0022X https:// doi. org/ 10. 1016/ B978-0- 12- 799937- 1. 00022-X 32. Mishra, T., & Pandey, V. C. Phytoremediation of red mud deposits through natural succession. In V. C. Pandey & K. Bauddh (Eds.), Phytomanagement of polluted sites (pp. 409–424). Elsevier (2019). https:// www. scien cedir ect. com/ scien ce/ artic le/ pii/ B9780 12813 91270 00168 https:// doi. org/ 10. 1016/ B978-0- 12- 813912- 7. 00016-8
33. Taylor, M., Kim, N., Smidt, G., McNally, S., Robinson, B., Kratz, S., & Schnug, E. Trace element contaminants and radioactivity from phosphate fertiliser. In E. Schnug & L. J. De Kok (Eds.), Phosphorus in agriculture: 100% zero (pp. 231–266) (2016). Springer. https:// doi. org/ 10. 1007/ 978- 94- 017- 7612-7_ 12
34. R Core Team. R: A language and environment for statistical computing (2021). https:// www.R- proje ct. org/.
35. Hothorn, T., Bretz, F. & Westfall, P. Simultaneous inference in general parametric models. Biometr. J. 50(3), 346–363 (2008). 36. Rafflegeau, S., Michel-Dounias, I., Tailliez, B., Ndigui, B. & Papy, F. Unexpected N and K nutrition diagnosis in oil palm smallholdings using references of high-yielding industrial plantations. Agron. Sustain. Dev. 30(4), 777–787. https:// doi. org/ 10. 1051/ agro/ 20100 19 (2010).
37. Esperschuetz, J. et al. Response of Leptospermum scoparium, Kunzea robusta and Pinus radiata to contrasting biowastes. Sci. Total Environ. 587–588, 258–265. https:// doi. org/ 10. 1016/j. scito tenv. 2017. 02. 134 (2017).
38. McLaren, R. G., & Cameron, K. C. Soil ccience: Sustainable production and environmental protection. Oxford University Press (1996). https:// books. google. co. nz/ books? id= AYVFA QAAIA AJ
39. Chew, P. S., & Teoh, K. C. Use of rachis analysis an indicator of K nutrient status in oil palm. International Oil Palm/Palm Oil Conference: Progress and Prospects, Kuala Lumpur (1987). 40. Cui, J., Lamade, E. & Tcherkez, G. Potassium deficiency reconfigures sugar export and induces catecholamine accumulation in oil palm leaves. Plant Sci. 300, 110628. https:// doi. org/ 10. 1016/j. plant sci. 2020. 110628 (2020).
41. Rankine, I. & Fairhurst, T. H. Management of phosphorus, potassium and magnesium in mature oil palm. Better Crops Int. 13(1), 10–15 (1999). 42. Jacquemard, J. C., H. Edyana, S., Dadang, K., & Tailliez, B. Expression of boron deficiency symptoms and link with the genotype in oil palm (Elaeis guineensis Jacq.) (2006). IOPC, Bali, Indonesia. 43. Aini Azura, A., Fauziah, C. I. & Samsuri, A. W. Cadmium and zinc concentrations in soils and oil palm tissues as affected by long-term application of phosphate rock fertilizers. Soil Sediment Contam. Int. J. 21(5), 586–603. https:// doi. org/ 10. 1080/ 15320 383. 2012. 672485 (2012). 44. El-Jaoual, T. & Cox, D. A. Manganese toxicity in plants. J. Plant Nutr. 21(2), 353–386. https:// doi. org/ 10. 1080/ 01904 16980 93654 09 (1998).
45. Mason, B. H., & Moore, C. B. (1982). Principles of geochemistry. Wiley. https:// books. google. co. nz/ books? id= K75gI AAACA AJ 46. Saleeb, N. et al. The mobility of silver nanoparticles and silver ions in the soil-plant system. J. Environ. Qual. 48(6), 1835–1841. https:// doi. org/ 10. 2134/ jeq20 19. 03. 0098 (2019).
47. Cowgill, U. M. The tellurium content of vegetation. Biol. Trace Elem. Res. 17(1), 43–67. https:// doi. org/ 10. 1007/ bf027 95446 (1988).
48. Akpanabiatu, M. I., Ekpa, O. D., Mauro, A. & Rizzo, R. Nutrient composition of Nigerian palm kernel from the dura and tenera varieties of the oil palm (Elaeis guineensis). Food Chem. 72(2), 173–177. https:// doi. org/ 10. 1016/ s0308- 8146(00) 00215-6 (2001).
49. Kok, S., Ong-Abdullah, M., Ee, G. C. & Namasivayam, P. Comparison of nutrient composition in kernel of tenera and clonal materials of oil palm (Elaeis guineensis Jacq.). Food Chem. 129(4), 1343–1347. https:// doi. org/ 10. 1016/j. foodc hem. 2011. 05. 023 (2011).
50. Mathews, J., Lee, A. K., Clarence, P. J., Chung, M. Y. & Rao, S. Oil content in oil palm fruit mesocarp and bunch, and some of its related physiological and agronomical factors. The Planter 80(938), 273–294 (2004).
51. Singh, P. K., Pratap, S. G., & Tandon, P. K. The mechanisms of trace element uptake and transport up to grains of crop plants. In Kumkum Mishra, Pramod Kumar Tandon, & S. Srivastava (Eds.), Sustainable solutions for elemental deficiency and excess in crop plants (pp. 119–133). Springer Singapore (2020).. https:// doi. org/ 10. 1007/ 978- 981- 15- 8636-1_6
52. Aladesanmi, O. T., Oroboade, J. G., Osisiogu, C. P. & Osewole, A. O. Bioaccumulation factor of selected heavy metals in Zea mays. J. Health Pollut. 9(24), 191207. https:// doi. org/ 10. 5696/ 2156- 9614-9. 24. 191207 (2019).
53. Reiser, R. et al. Cadmium concentrations in New Zealand pastures: Relationships to soil and climate variables. J. Environ. Qual. 43(3), 917–925. https:// doi. org/ 10. 2134/ jeq20 13. 09. 0367 (2014).
54. Chalil, D. Market power and subsidies in the Indonesian palm oil industry AARES 52nd Annual conference, Canberra, Australia (2008). https:// doi. org/ 10. 22004/ ag. econ. 6022 https:// doi. org/ 10. 22004/ ag. econ. 6022
55. Ouerdane, L., Mari, S., Czernic, P., Lebrun, M. & Łobiński, R. Speciation of non-covalent nickel species in plant tissue extracts by electrospray Q-TOFMS/MS after their isolation by 2D size exclusion-hydrophilic interaction LC (SEC-HILIC) monitored by ICP-MS. J. Anal. At. Spectrom. 21(7), 676–683. https:// doi. org/ 10. 1039/ b6026 89c (2006).
56. Almeida, M. & Carpenter, K. Determining trace elements in edible oils using inductively coupled plasma–optical emission spectrometry. Spectrosc. Suppl. Special Issues 30(11), 26–31 (2015).
57. Perlein, A. et al. Phytomanagement of a metal(loid)-contaminated agricultural site using aromatic and medicinal plants to produce essential oils: analysis of the metal(loid) fate in the value chain. Environ. Sci. Pollut. Res. 28(44), 62155–62173. https:// doi. org/ 10. 1007/ s11356- 021- 15045-4 (2021).
58. Obi, A. L., Jonah, S. A. & Umar, I. Determination of trace elements in some Nigerian vegetable based oilsby neutron activation analysis. J. Radioanal. Nucl. Chem. 249(3), 669–671. https:// doi. org/ 10. 1023/a: 10132 31222 908 (2001).
59. Nnorom, I. C., Alagbaoso, J. E., Amaechi, U. H., Kanu, C. & Ewuzie, U. Determination of beneficial and toxic metals in fresh palm oil (Elaeis guineensis Jacq.) from south-eastern Nigeria: Estimation of dietary intake benefits and risks. J. Sci. Res. Rep. 3(16), 2216–2226 (2014).
60. Asemave, K., Ubwa, S. T., Anhwange, B. A. & Gbaamende, A. G. Comparative evaluation of some metals in palm oil, groundnut oil and soybean oil from Nigeria. Int. J. Mod. Chem. 1(1), 28–35 (2012).
61. Otten, J. J., Hellwig, J. P., & Linda D. Meyers. (2006). Dietary reference intakes: The essential guide to nutrient requirements. National Academies Press. https:// www. nal. usda. gov/ sites/ defau lt/ files/ fnic_ uploa ds/ DRIEs senti alGui deNut Req. pdf
62. Zhao, X. et al. Studying the evaluation model of the nutritional quality of edible vegetable oil based on dietary nutrient reference intake. ACS Omega 6(10), 6691–6698. https:// doi. org/ 10. 1021/ acsom ega. 0c055 44 (2021).
63. Hinton, T.G., Kopp, P., Ibrahim, S., Bubryak, I., Syomov, A., Tobler, L., Bell, C., 1995. A comparison of techniques used to estimate the amount of resuspended soil on plant surfaces. Health Phys. 68, 523e531.
64. Benning, U., Tamot, B., Guelette, B., & Hoffmann-Benning, S. (2012, 2012-March-28). New aspects of phloem-mediated long-
distance lipid signaling in plants [Hypothesis and Theory]. Front. Plant Sci. https:// doi. org/ 10. 3389/ fpls. 2012. 00053
65. Aguilar, F. et al. Safety of aluminium from dietary intake - scientific opinion of the panel on food additives, flavourings, processing aids and food contact materials (afc). EFSA J. https:// doi. org/ 10. 2903/j. efsa. 2008. 754 (2008).
66. FAO/WHO. (2000). Safety evaluation of certain food additives and contaminants (WHO Food Additives Series, Issue. WHO/FAO. https:// inchem. org/ docum ents/ jecfa/ jecmo no/ v44je c12. htm
67. FAO/WHO. (2004). Evaluation of certain food additives and contaminants (WHO Techncial Report Series—922, Issue. WHO. https:// apps. who. int/ iris/ bitst ream/ handle/ 10665/ 42849/ WHO_ TRS_ 922. pdf? seque nce= 1& isAll owed=y
68. Njoku, P. C., Egbukole, M. O. & Enenebeaku, C. K. Physio-chemical characteristics and dietary metal levels of oil from elaeis guineensis species. Pak. J. Nutr. 9(2), 137–140. https:// doi. org/ 10. 3923/ pjn. 2010. 137. 140 (2010).
69. Adepoju-Bello, A. A., Osagiede, S. A. & Oguntibeju, O. O. Evaluation of the concentration of some toxic metals in dietary red palm oil. J. Bioanal. Biomed. 4(50), 92–95 (2012).
70. Aigberua, A. O., Ovuru, K. F. & Izah, S. C. Evaluation of selected heavy metals in palm oil sold in some markets in Yenagoa metropolis, Bayelsa State, Nigeria. E C Nutr. 11(6), 244–252 (2017).
71. Chen, S. S., Lee, B. Y., Cheng, C. C. & Chou, S. S. Determination of arsenic in edible fats and oils by focused microwave digestion and atomic fluorescence spectrometer. J. Food Drug Anal. 9(2), 121–125 (2001).
72. Chen, S. S., Cheng, C. C. & Chou, S. S. Determination of arsenic in edible fats and oils by direct grahite furnace atomic absorption spectrometry. J. Food Drug Anal. 11(3), 214–219 (2003).
6Author contributions作者贡献
H. T.-M. Writing—original draft, formal analysis, visualisation. F. A. Resources, writing—review and editing. S. M. A. Resources, writing—review and editing. S. G. Writing—review and editing, supervision. B. R. Writing—review and editing, supervision.
H. T.-M.:撰写—初稿、形式分析、可视化。F. A.:资源、撰写—审阅与编辑。S. M. A.:资源、撰写—审阅与编辑。S. G.:撰写—审阅与编辑、指导。B. R.:撰写—审阅与编辑、指导。
7Funding基金资助
This work was supported by A Well Fed World; The Centre for Integrated Biowaste Research funded by Strategic Science Investment Funding from Ministry of Business, Innovation and Employment, New Zealand (contract C03X1701); and a University of Canterbury Doctoral Scholarship.
本研究由A Well Fed World、新西兰商业、创新与就业部战略科学投资基金资助的综合生物废弃物研究中心(The Centre for Integrated Biowaste Research,合同号C03X1701)以及坎特伯雷大学博士奖学金资助。
8Competing interests利益冲突
The authors declare no competing interests.
作者声明不存在利益冲突。
9Additional information附加信息
Supplementary Information The online version contains supplementary material available at https:// doi. org/ 10. 1038/ s41598- 023- 50492-8.
补充信息 在线版本包含补充材料,网址为https:// doi. org/ 10. 1038/ s41598- 023- 50492-8。
Correspondence and requests for materials should be addressed to H.T.-M.
通讯作者:索取材料请联系H.T.-M.。
Reprints and permissions information is available at www.nature.com/reprints.
重印及许可信息见www.nature.com/reprints。
Publisher’s note Springer Nature remains neutral with regard to jurisdictional claims in published maps and institutional affiliations.
出版者声明 Springer Nature对已出版地图中的管辖权主张及机构隶属关系保持中立。
Open Access This article is licensed under a Creative Commons Attribution 4.0 International License, which permits use, sharing, adaptation, distribution and reproduction in any medium or format, as long as you give appropriate credit to the original author(s) and the source, provide a link to the Creative Commons licence, and indicate if changes were made. The images or other third party material in this article are included in the article’s Creative Commons licence, unless indicated otherwise in a credit line to the material. If material is not included in the article’s Creative Commons licence and your intended use is not permitted by statutory regulation or exceeds the permitted use, you will need to obtain permission directly from the copyright holder. To view a copy of this licence, visit http:// creat iveco mmons. org/ licen ses/ by/4. 0/.
开放获取 本文采用知识共享署名4.0国际许可协议(Creative Commons Attribution 4.0 International License)授权,该协议允许以任何媒介或格式使用、共享、改编、分发和复制本文,但须适当注明原作者及来源,提供知识共享许可协议的链接,并说明是否作了修改。除非在材料的署名说明中另有注明,本文中的图像或其他第三方材料均包含在本文的知识共享许可协议中。如果材料未包含在本文的知识共享许可协议中,且您的预期用途不为法律法规所允许或超出允许的使用范围,则需直接获得版权持有人的许可。如需查看该许可协议的副本,请访问 http:// creat iveco mmons. org/ licen ses/ by/4. 0/。
© The Author(s) 2024